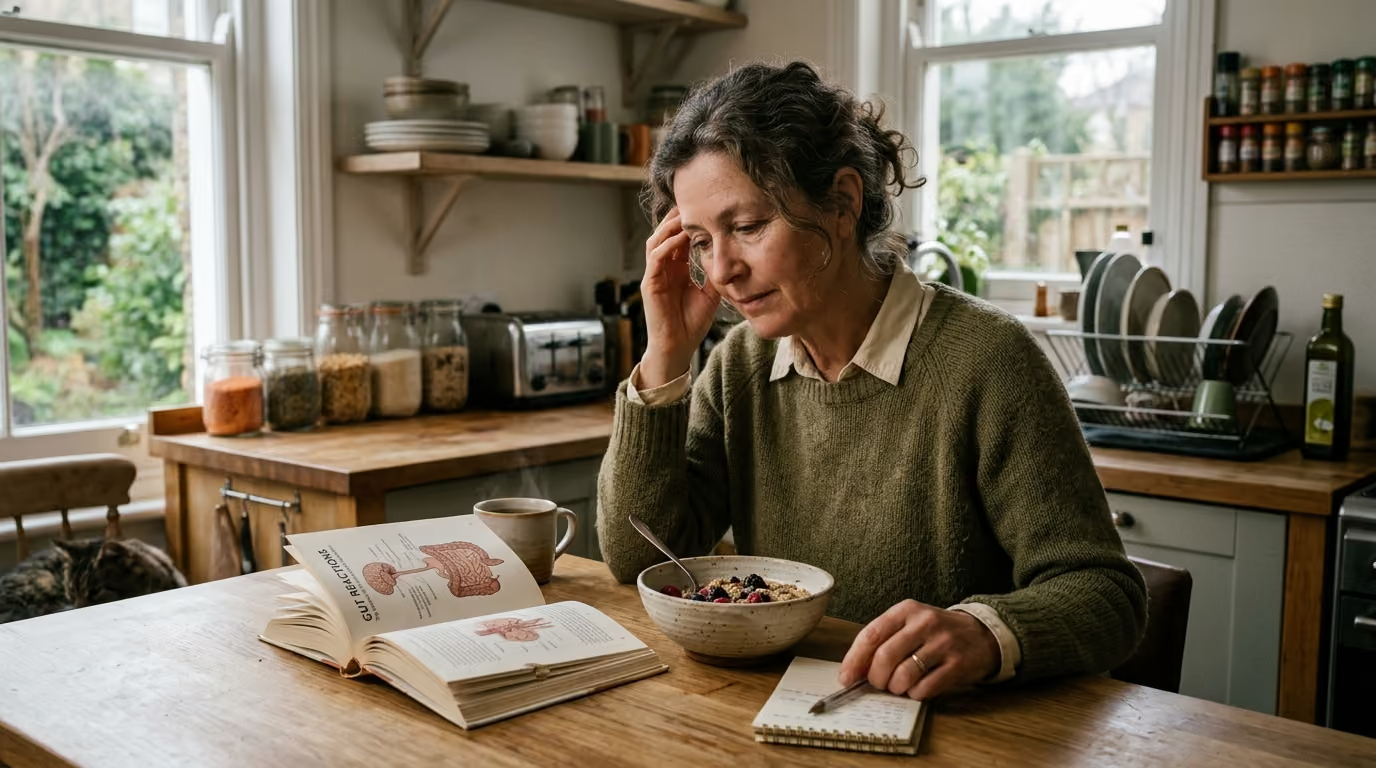
Finishing a large meal triggers vital gut-brain communication pathways that regulate appetite, vagus nerve activity, and long-term metabolic health across complex biological systems.


Many people assume appetite and metabolic health are governed solely by conscious willpower or simple calorie arithmetic. When hunger strikes or energy levels drop, conventional advice often treats the brain as the master controller and the stomach as an empty container waiting for fuel. Biological research reveals a very different reality.
Metabolism is regulated through a continuous, two-way communication network linking the gastrointestinal tract and the central nervous system. Every meal triggers a cascade of neural impulses, peptide hormones, and microbial metabolites that inform the brain about nutrient availability. Yet, while commercial wellness culture often claims that altering a single gut microbe can instantly change body weight, scientific realities are far more nuanced. Understanding the true scope of gut-brain connection and whole-body wellness requires distinguishing between laboratory mechanisms, population trends, and what actually applies to an individual.
The scientific consensus recognizes the gut-brain axis as a bidirectional communication highway. It connects the gastrointestinal system directly to cognitive and autonomic centers in the brain. This network does not rely on a single physical pathway. Instead, it operates through an integrated system of neural circuits, endocrine signals, immune responses, and metabolic byproducts.
Signals move in both directions continuously. The gut informs the brain about the physical presence, volume, and chemical composition of food in the digestive tract. In response, the brain modulates gut motility, fluid secretion, barrier integrity, and the release of digestive enzymes. Through these coordinated pathways, the gut-brain axis helps manage short-term feelings of fullness, long-term energy balance, and systemic glucose regulation.
Mechanistic studies in animal models have revealed many biological pathways showing how intestinal events influence brain centers. Researchers can observe specific nerve fibers firing when nutrients touch the intestinal lining. They can also track how peptide hormones cross physiological barriers to influence appetite centers in the hypothalamus and brainstem.
However, major health organizations and research bodies urge caution when translating these findings to human health. Demonstrating that a pathway exists in an animal model does not prove it governs everyday human metabolism. Furthermore, observing a statistical correlation in a large population study does not mean that modifying that pathway will produce predictable metabolic changes for a specific person.
Evidence firmly establishes that gut-brain signaling is essential for metabolic regulation. Yet science has not established that stool tests or targeted microbial supplements can reliably diagnose or correct individual metabolic concerns.
To understand how the digestive tract influences metabolic health, one must examine the physical structures and chemical messengers involved in the process. The gut uses several parallel systems to monitor incoming nutrients and relay that data to the nervous system.
The lining of the gastrointestinal tract contains specialized sensory cells known as enteroendocrine cells. Although they make up less than one percent of the intestinal epithelial cell layer, they play a massive role in sensing food. As carbohydrates, fats, and proteins break down during digestion, these cells detect specific macronutrients using specialized surface receptors.
When activated, enteroendocrine cells release signaling peptides into surrounding tissues and the bloodstream. These peptides include:
None of these hormones operate in isolation. They form a dynamic, overlapping communication network that adjusts continuously during and after a meal.
The vagus nerve serves as the primary physical bridge connecting the abdominal organs to the brainstem. Vagal sensory fibers, known as afferents, extend throughout the layers of the stomach and intestines. These nerve endings sit close to enteroendocrine cells, smooth muscle layers, and mucosal surfaces.
When food enters the stomach and small intestine, physical stretch receptors activate vagal afferents to report mechanical distension. Simultaneously, gut peptides like CCK and GLP-1 bind to receptors on these same nerve endings. The vagus nerve converts these chemical and mechanical cues into electrical impulses. These impulses travel directly to the nucleus of the solitary tract in the brainstem, which relays information to higher brain regions that regulate hunger, satisfaction, and autonomic output.
Disrupting vagal afferent signaling in laboratory experiments reduces an animal's sensitivity to intestinal nutrients. This disruption alters immediate meal sizes and changes how brainstem circuits respond to food intake. These findings prove that the vagus nerve is an indispensable component of nutrient sensing. However, vagal signaling is only one part of the gut-brain axis. Hormones circulating through the bloodstream and immune signaling molecules also communicate directly with the brain, independent of the vagus nerve.
The trillions of microorganisms residing in the large intestine contribute their own chemical signals to this network. When gut microbes ferment non-digestible dietary fibers, they produce short-chain fatty acids (SCFAs). The three most abundant SCFAs are acetate, propionate, and butyrate.
These fatty acids serve as local fuel sources for colon cells and act as signaling molecules throughout the body. SCFAs can bind to free fatty acid receptors located on enteroendocrine cells, immune cells, and autonomic nerve terminals. Through these receptor interactions, microbial metabolites may stimulate the release of satiety-promoting hormones like GLP-1 and PYY.
While this microbial mechanism is biologically plausible, the strength and consistency of these signals vary significantly based on diet, transit time, and individual physiology.
Discussions surrounding gut health and metabolism often blend several distinct biological concepts together. Popular wellness resources frequently treat hunger ratings, daily food intake, body weight, and metabolic health as if they were identical measurements. Scientific research treats each of these endpoints as separate phenomena that require independent evaluation.
Appetite is a subjective sensation. Clinical studies often measure appetite using visual analog scales where participants rate their feelings of hunger, fullness, and desire to eat at specific intervals. While these self-reported ratings offer valuable clues about short-term satisfaction, they do not always correlate with actual food consumption.
A person may report feeling fuller after consuming a specific nutrient or fiber supplement without actually reducing the total number of calories they eat during an unrestricted meal. Conversely, an individual might consume fewer calories during an experimental test meal due to gastrointestinal discomfort rather than genuine physiological fullness. Researchers must measure both subjective appetite scores and real-world caloric intake to determine whether a gut signal meaningfully alters eating behavior.
Observing that a gut-derived signal reduces food intake during a single laboratory meal does not prove that it will cause long-term weight changes. The human body possesses redundant, compensatory metabolic systems designed to protect energy stores.
If a dietary intervention lowers caloric intake during breakfast, the body may compensate by increasing hunger signals later in the evening or reducing non-exercise physical activity. Long-term body weight is shaped by cumulative energy balance over months and years, alongside genetic, environmental, and behavioral influences. Short-term satiety experiments provide helpful physiological data, but they cannot serve as stand-alone evidence for sustained changes in body weight or body composition.
Body weight alone is an incomplete marker of overall metabolic health. An individual can carry excess adipose tissue while maintaining normal insulin sensitivity, healthy blood lipid levels, and stable blood pressure. Conversely, a person with a standard body mass index may experience impaired glucose tolerance, hepatic steatosis, or chronic low-grade systemic inflammation.
Research examining digestion and everyday gut function looks beyond body weight. Scientists evaluate glycemic variability, postprandial lipid handling, liver fat accumulation, and inflammatory markers. Gut-brain signaling influences many of these parameters simultaneously. For instance, GLP-1 release alters post-meal blood glucose clearance through its actions on the pancreas, regardless of whether it leads to noticeable weight changes. Evaluating metabolic wellbeing requires looking at systemic metabolic markers rather than focusing solely on a bathroom scale.
Short-chain fatty acids are often portrayed as a direct bridge linking diet, the microbiome, and metabolic wellness. Because these molecules are produced when bacteria ferment dietary fiber, many theories suggest that increasing SCFA production will naturally suppress appetite and improve metabolic markers. A closer look at human clinical trials reveals a much more nuanced picture.
In cell cultures and animal models, SCFAs display clear metabolic benefits. When applied directly to isolated intestinal tissues, acetate, propionate, and butyrate trigger the secretion of GLP-1 and PYY. In rodent studies, infusing SCFAs into the digestive tract often leads to reduced food intake, improved insulin sensitivity, and protection against diet-induced weight gain.
However, clinical trials in humans have produced mixed results. The effects of SCFAs in people depend heavily on the delivery method, the specific molecule tested, and the location in the digestive tract where exposure occurs.
For example, a comprehensive review of human and animal studies examined the effects of oral propionate on eating behavior. In one human study, oral administration of propionate did not alter total energy intake during an unrestricted test meal, nor did it change energy intake over the subsequent 24 hours. While animal models showed clear appetite suppression, the same response did not reliably occur when humans consumed the compound orally.
The site where SCFAs are released or administered plays a fundamental role in how the body processes them. Under normal physiological conditions, microbial fermentation takes place primarily in the cecum and colon. The concentration of SCFAs is highest in the proximal large intestine and decreases steadily toward the rectum.
When humans consume oral SCFA salts, the compounds are rapidly absorbed in the stomach and upper small intestine. This rapid absorption differs dramatically from the gradual, continuous production that occurs when complex carbohydrates undergo microbial fermentation in the colon.
Some clinical protocols use targeted delivery capsules or colonic infusions to bypass the upper digestive tract. While these specialized methods occasionally show modest increases in circulating gut hormones or slight reductions in acute energy intake, results vary widely between participants.
Evidence does not support the idea that simply having more SCFAs in the gut leads directly to reduced appetite or sustained weight loss. These molecules act as subtle modulators within a complex biological system, not as universal switches for metabolic control.
A major goal in commercial microbiome science is personalized nutrition. The concept suggests that analyzing the bacterial strains in a person's stool sample can predict how their metabolism will respond to specific diets. While population-level research has identified intriguing associations, translating those findings into individualized dietary guidance remains challenging.
One widely studied microbiome pattern involves the balance between two dominant bacterial genera: Prevotella and Bacteroides. Several cohort studies observed that participants with a higher baseline abundance of Prevotella relative to Bacteroides lost more weight on high-fiber, whole-grain diets than individuals with lower Prevotella levels.
This finding generated significant enthusiasm for using baseline stool tests to match individuals with specific weight-management plans. However, subsequent clinical reviews have reached more cautious conclusions. When researchers attempt to replicate these findings across diverse populations with varying backgrounds and eating patterns, the predictive relationship often weakens or disappears entirely.
Systematic reviews evaluating the available literature conclude that evidence remains insufficient to claim a person's baseline microbiome can reliably predict their weight-loss response to a high-fiber diet.
Long-term intervention studies continue to highlight the difficulty of using gut bacteria as predictive markers. In one rigorous dietary trial, researchers tracked participants with overweight or obesity assigned to either a healthy low-carbohydrate diet or a healthy low-fat diet over twelve months. The study analyzed baseline microbiome composition as well as microbial changes occurring at three months and twelve months.
The trial yielded several critical insights:
These findings demonstrate that while diets rich in food, fiber, and varied nutrition reliably support metabolic health across broad groups, a baseline stool profile cannot tell an individual which dietary approach will work best for their biology.
Some recent research papers use machine-learning algorithms to build predictive models of weight loss based on multi-omic gut profiles. For example, a 2026 scientific review analyzed a predictive model that achieved an internally cross-validated area under the receiver operating characteristic curve (AUC) of 0.80 for identifying individuals who reached a specific weight-loss threshold.
While an AUC of 0.80 appears statistically strong, the underlying study included only 46 total participants who completed the protocol, with just 14 individuals actually reaching the target weight-loss threshold. Furthermore, the mathematical model was never tested or validated in an independent, external cohort of patients.
Similarly, a sub-study from the large-scale PREVIEW trial reported that baseline microbiota features accounted for roughly 25 percent of the variation in body-fat changes during an eight-week low-energy diet. While scientifically valuable for generating new hypotheses, a statistical correlation explaining one-quarter of variance in a tightly controlled trial cannot serve as a reliable forecast for a single person navigating everyday life.
Commercial tests that claim to predict metabolic outcomes based on stool samples consistently outpace the established science.
Misinformation regarding digestive wellness is widespread. Oversimplified narratives often transform nuanced physiological concepts into exaggerated wellness claims. Clarifying these misunderstandings helps create a realistic, evidence-aware understanding of gut-brain signaling.
Direct-to-consumer testing companies frequently suggest that mapping your gut microbiome will pinpoint the exact reason you struggle with blood glucose spikes, food cravings, or weight management. This claim misrepresents what stool tests actually measure.
A standard microbiome test provides a single snapshot of the bacterial DNA fragments present in a stool sample. It cannot measure dynamic gut-brain signaling, real-time hormone release, vagal nerve sensitivity, or intestinal mucosal health.
Furthermore, having a microbial composition associated with metabolic dysfunction in a population study does not mean those bacteria are causing your personal metabolic patterns. Genetic background, physical activity, sleep patterns, emotional stress, and daily nutrition exert far more direct control over metabolic health than the presence or absence of specific bacterial strains.
Marketing for probiotic supplements often describes an ideal, universal microbiome that promotes leanness and metabolic efficiency. Science shows that no such single profile exists.
Healthy, metabolically fit individuals across different global populations display widely varying gut microbiomes. Indigenous hunter-gatherer populations, agrarian communities, and urban populations possess completely different bacterial ecosystems, yet individuals within all these groups can maintain robust metabolic health.
Metabolic wellness is supported by functional capacity rather than a rigid list of specific bacterial species. A diverse ecosystem capable of fermenting various fibers, maintaining intestinal barrier integrity, and synthesizing essential vitamins can look entirely different from one person to the next.
Media coverage of metabolic medications often portrays individual gut peptides, particularly GLP-1 or ghrelin, as independent switches controlling hunger. In reality, human appetite is regulated through an intricate web of overlapping, redundant systems.
If circulating levels of one satiety peptide rise, the body may adjust by altering the sensitivity of peripheral receptors, changing gastric motility, or modulating central reward pathways in the brain. Psychological context, visual food cues, circadian rhythms, and learned meal routines also influence hunger independently of immediate gut hormone concentrations.
No single hormone acts as an absolute controller of human eating behavior. Natural appetite regulation depends on the coordinated harmony of dozens of simultaneous signals.
Much of the popular belief that gut microbes directly drive body weight stems from early rodent experiments. In widely cited studies, researchers transferred fecal microbiota from human twins with discordant body weights into germ-free mice. The mice that received microbes from the twin with obesity gained more body fat than mice receiving microbes from the twin without obesity, despite eating identical amounts of food.
While these experiments provided ground-breaking mechanistic insights in a controlled laboratory setting, they cannot be directly applied to human health. Germ-free mice are raised in completely sterile environments and lack normally developed immune and metabolic systems.
Subsequent clinical reviews have highlighted that human fecal microbiota transplants (FMT) have failed to replicate these dramatic body-composition changes in human recipients. Human energy balance and metabolism are governed by far more complex host physiology, habitual diet, and lifestyle behaviors than the biology of a germ-free mouse.
While oversimplified marketing should be viewed with healthy skepticism, legitimate scientific research into the gut microbiome and digestive science continues to uncover fascinating biological insights. Scientists are exploring how gut-brain communication works at the cellular and molecular levels.
For decades, scientists believed that enteroendocrine cells communicated with the nervous system exclusively through slow, hormonal release into the bloodstream. Groundbreaking research has identified a specialized subtype of enteroendocrine cells called "neuropod cells."
These cells possess physical, axon-like extensions that form direct synaptic connections with nearby vagal nerve endings. Instead of relying solely on hormonal diffusion over minutes or hours, neuropod cells can transmit sensory information about glucose and other nutrients to the brainstem in milliseconds using neurotransmitters like glutamate.
This rapid-fire signaling mechanism allows the brain to perceive the chemical contents of the gut almost instantaneously. Researchers are currently investigating how this rapid pathway interacts with slower hormonal feedback to regulate real-time food choices and meal termination.
Another promising area of metabolic research focuses on bile acids as active signaling molecules. Synthesized in the liver and released into the small intestine to aid fat digestion, primary bile acids travel to the distal gut, where resident microbes convert them into secondary bile acids.
These transformed bile acids bind to specific host receptors, including the farnesoid X receptor (FXR) and the G-protein coupled bile acid receptor 1 (TGR5). Activation of TGR5 on enteroendocrine L-cells promotes the secretion of GLP-1, while FXR activation in liver and gut tissues influences systemic lipid metabolism and hepatic glucose handling.
This bile-acid pathway represents a true three-way interaction between host physiology, microbial metabolism, and systemic energy regulation. Scientists are working to determine whether therapeutic compounds targeting these receptors can help manage non-alcoholic fatty liver disease and insulin resistance.
Often referred to as the "second brain," the enteric nervous system (ENS) contains hundreds of millions of neurons embedded directly within the walls of the gastrointestinal tract. While the vagus nerve handles long-distance communication with the brainstem, the ENS manages local gut reflexes independently.
Recent investigations demonstrate that enteric neurons communicate constantly with nearby immune cells, mucosal epithelial cells, and microbial populations. Enteric neural circuits monitor mechanical tension, chemical irritation, and local inflammation, altering intestinal permeability and blood flow in response.
Understanding how the ENS coordinates with systemic metabolic pathways represents a vital frontier in gastroenterology and metabolic research.
Supporting the biological communication networks between your gut and brain does not require costly supplements or extreme dietary restrictions. Scientific evidence consistently shows that everyday, sustainable lifestyle habits create the best physiological environment for healthy digestive signaling and metabolic stability.
Rather than searching for a single specialized food, focus on providing a wide variety of fermentable carbohydrates to support diverse microbial communities. Different types of dietary fiber serve as substrates for different microbial species, leading to a balanced production of beneficial metabolites like acetate, propionate, and butyrate.
Practical ways to build dietary diversity include:
Because chemical and mechanical gut-brain signaling takes time to register in the central nervous system, eating too quickly can lead to consuming excess energy before satiety hormones have reached peak circulation.
Allowing 20 to 30 minutes to finish a balanced meal provides sufficient time for gastric stretch receptors and enteroendocrine L-cells to release CCK, PYY, and GLP-1. Simple behavioral adjustments, such as chewing food thoroughly, setting down utensils between bites, and minimizing screen-based distractions during meals, help you tune into natural physiological fullness cues.
Both the gastrointestinal tract and metabolic organs operate on internal 24-hour circadian clocks. Intestinal motility, digestive enzyme secretion, gastric acid production, and glucose tolerance all follow distinct daily rhythms, peaking during daylight hours and slowing during the night.
Irregular sleep schedules, late-night eating, and shift work can disrupt these peripheral clocks, impairing gut-brain signaling and reducing insulin sensitivity. Maintaining consistent sleep and wake times, alongside consuming the majority of your daily calories during daylight hours, helps synchronize your metabolic systems and supports digestive harmony.
Engaging in regular, moderate physical activity offers substantial metabolic and digestive benefits. Exercise enhances peripheral insulin sensitivity in skeletal muscle tissue, stimulates healthy colonic motility, and supports gut barrier integrity.
Activities like brisk walking, cycling, swimming, or resistance training promote metabolic health independently of changes on the scale. Combining consistent movement with a nutrient-rich, fiber-diverse diet creates the optimal biological foundation for the gut-brain axis to function effectively.
While lifestyle and nutritional adjustments support general digestive wellness, they are not appropriate substitutes for medical care when significant symptoms arise. Digestive and metabolic concerns can sometimes point to underlying clinical conditions that require professional diagnosis and targeted treatment.
If you experience any of the following symptoms, schedule a prompt evaluation with a qualified physician or gastroenterologist:
If you have ongoing concerns about blood sugar regulation, persistent metabolic challenges, or recurring gastrointestinal discomfort, seek guidance from registered dietitians, gastroenterologists, or endocrinologists. These licensed professionals rely on validated diagnostic tools, such as comprehensive blood panels, endoscopic imaging, and standardized breath tests, rather than unvalidated direct-to-consumer kits.
Working with a healthcare professional ensures you receive a personalized, evidence-based care plan tailored to your medical history and biological needs. You can learn more about DigestGenius and our commitment to providing clear, research-led educational resources.
Understanding how your digestive tract communicates with your brain empowers you to make informed, realistic choices that support lifelong metabolic wellness.
DigestGenius publishes research-led guidance on digestion, the gut microbiome, fiber, probiotics, gut-brain signaling, inflammation and everyday digestive wellbeing.


Explore clear, research-led guidance on digestion, the microbiome, food, fiber, probiotics and the gut-brain connection.
read the blog